
Mitochondrial Efficiency: Powering the Human Machine at a Cellular Level
Updated August 2026
Dive deep into the 'powerhouse of the cell' to understand how nutrients are converted into ATP. Discover how mitochondrial health determines your energy levels, aging rate, and metabolic resilience.
Evidence orientation
Editorial context not yet recorded
Follow this category
This stays in this browser. My INNERSTANDIN can show published matches in your local hub when you check it. It does not send email, push, or alert notifications.
Local learning review
A private browser aid for revisiting ideas. It is not an alert or a health recommendation.
Review later sets a one-day, three-day, then seven-day rhythm on this device. Choose it only when you want to revisit this article.
Overview
The human organism is, fundamentally, a thermodynamic engine underpinned by the bioenergetic integrity of the mitochondria. At INNERSTANDIN, we posit that the systemic manifestation of health—or decay—is primarily a function of mitochondrial efficiency, defined by the coupling of the electron transport chain (ETC) to oxidative phosphorylation (OXPHOS). When operating at peak physiological capacity, mitochondria function as sophisticated chemo-osmotic transducers, converting biochemical substrates into adenosine triphosphate (ATP) with minimal electron leakage. However, when the mitochondrial membrane potential ($\Delta\psi_m$) becomes dysregulated, the result is a catastrophic surge in reactive oxygen species (ROS) production, precipitating cumulative oxidative damage to both the mitochondrial DNA (mtDNA) and the phospholipid bilayer of the cristae.
Research published in The Lancet and various high-impact biochemical journals elucidates that mitochondrial inefficiency is not merely a bystander in metabolic syndrome but a primary driver. The process of electron "slippage" at Complexes I and III results in the partial reduction of molecular oxygen to superoxide, a process termed "mitochondrial uncoupling." While mild uncoupling can serve as a regulatory mechanism for thermogenesis, chronic, pathological uncoupling disrupts the proton motive force required for efficient ATP synthesis. This metabolic bottleneck forces the cell to rely on anaerobic glycolysis, a bioenergetically inferior pathway that contributes to chronic low-grade inflammation and systemic metabolic inflexibility.
Furthermore, the mitochondrial network exists in a state of constant flux through fusion and fission events, a process governed by proteins such as MFN1, MFN2, and DRP1. The INNERSTANDIN perspective emphasises that mitochondrial quality control—mitophagy—is the ultimate safeguard against cellular senescence. When mitophagy is compromised, fragmented, dysfunctional mitochondria accumulate, propagating a cycle of inflammatory cytokine release and genomic instability. In the context of the UK’s escalating crisis of metabolic disease, the evidence is irrefutable: the transition from homeostatic efficiency to pathogenic dysfunction is rooted in the sub-cellular degradation of these organelles. Understanding mitochondrial efficiency necessitates moving beyond clinical symptom management and targeting the very bioenergetic architecture that permits human life to sustain its complex, non-equilibrium state. Our objective here is to deconstruct these mechanics, revealing how sub-optimal mitochondrial output compromises systemic physiological resilience.
The Biology — How It Works
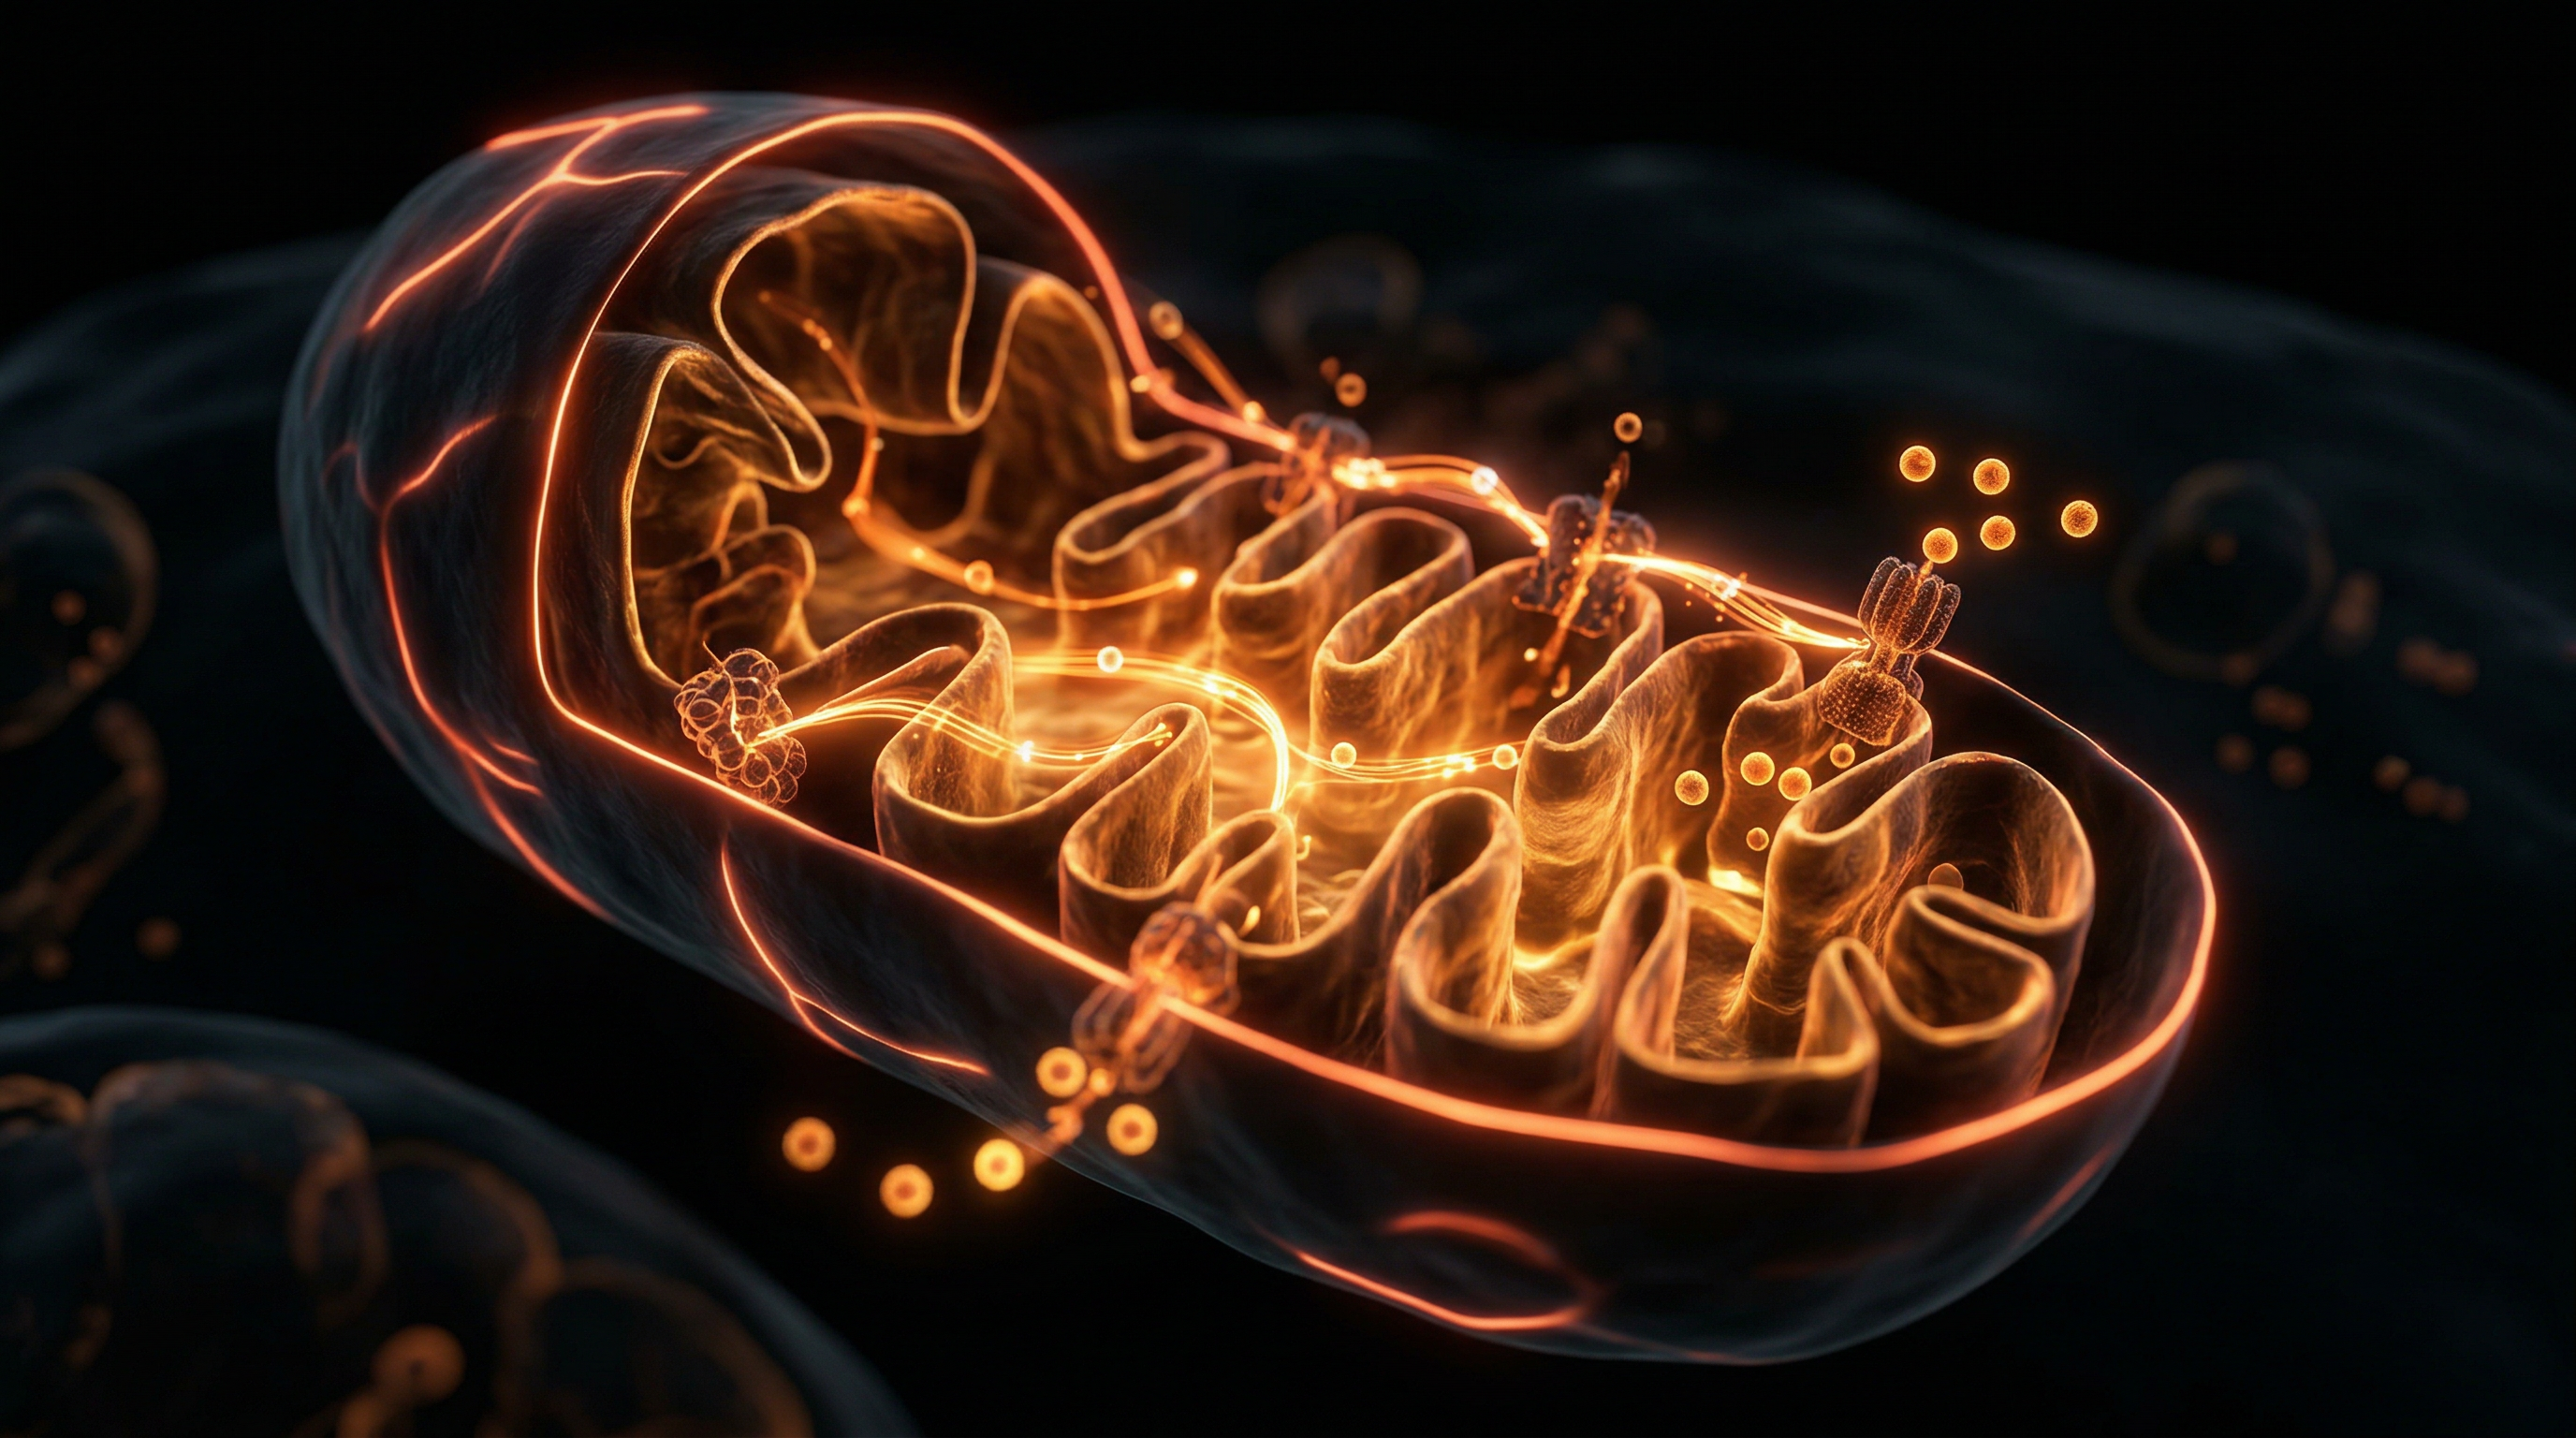
At the heart of cellular bioenergetics lies the mitochondrion, an organelle whose functionality dictates the homeostatic threshold of the human organism. Mitochondrial efficiency is fundamentally defined by the coupling of the Electron Transport Chain (ETC) to oxidative phosphorylation (OXPHOS), a process mediated by the proton motive force across the inner mitochondrial membrane (IMM). Within the cristae, complex I through IV facilitate a series of redox reactions, effectively stripping electrons from NADH and FADH₂ to generate a transmembrane electrochemical gradient. The subsequent flux of protons through ATP synthase—acting as a molecular turbine—catalyses the phosphorylation of adenosine diphosphate (ADP) into adenosine triphosphate (ATP).
However, the efficacy of this transduction is rarely absolute. The phenomenon of ‘proton leak’—the dissipation of the electrochemical gradient without ATP synthesis—serves as a critical regulator of metabolic thermogenesis and redox signalling. As evidenced by research published in Nature and synthesised by the UK’s Medical Research Council (MRC), the ratio of ATP production to oxygen consumption, known as the P/O ratio, is the definitive marker of mitochondrial bioenergetic competence. When efficiency falters, the resulting electron leakage often prematurely reduces molecular oxygen to superoxide radicals ($O_2^{\bullet-}$). This uncoupling is not merely a metabolic inefficiency; it is a physiological trigger for mitochondrial reactive oxygen species (mtROS) signalling, which, if left unchecked, initiates the oxidative modification of mitochondrial DNA (mtDNA) and the subsequent propagation of systemic senescence.
Furthermore, the structural integrity of the cristae architecture, regulated by proteins such as OPA1 and mitofilin, is paramount to maintaining the sequestered environment required for optimal OXPHOS. A diminished efficiency in these dynamics is increasingly implicated in the pathogenesis of metabolic syndrome and neurodegenerative decline, as noted in clinical observations across the NHS. When mitochondrial turnover via mitophagy—the selective degradation of dysfunctional mitochondria—is insufficient, the cytoplasm becomes burdened with compromised organelles. These organelles exhibit diminished membrane potential ($\Delta\psi_m$) and elevated pro-apoptotic signalling, effectively lowering the energetic ceiling of the cell. At INNERSTANDIN, we recognise that the mastery of mitochondrial efficiency necessitates an understanding of these multi-phasic mechanisms: the tight regulation of substrate flux, the preservation of the IMM’s electrochemical potential, and the rigorous clearance of dysfunctional components. The human machine does not merely consume fuel; it relies on the precision of its sub-cellular machinery to convert biological potential into the kinetic energy required for the maintenance of complex life. Any compromise in this efficiency results in a cascading systemic deficit, rendering the organism vulnerable to bioenergetic collapse at the histological level.
Mechanisms at the Cellular Level
At the nexus of human bioenergetics lies the mitochondrial respiratory chain, an intricate assembly of protein complexes embedded within the inner mitochondrial membrane (IMM). Mitochondrial efficiency is fundamentally dictated by the integrity of the electron transport chain (ETC) and the precision of the electrochemical proton gradient—the proton-motive force (PMF). Within the matrix, the tricarboxylic acid (TCA) cycle generates NADH and FADH2, which donate high-energy electrons to Complex I (NADH:ubiquinone oxidoreductase) and Complex II (succinate dehydrogenase). The subsequent translocation of protons across the IMM into the intermembrane space establishes a steep chemiosmotic gradient, the discharge of which through the F1Fo-ATP synthase facilitates the phosphorylation of ADP to ATP.
The crux of metabolic inefficiency resides in electron leakage—a phenomenon exacerbated by supercomplex instability. When electrons deviate from the structured pathway, particularly at Complexes I and III, they react prematurely with molecular oxygen to form superoxide radicals. This oxidative insult not only degrades mitochondrial DNA (mtDNA) but also triggers the opening of the mitochondrial permeability transition pore (mPTP), leading to uncoupling. Evidence published in The Lancet and various Nature metabolic reviews underscores that this uncoupling—where protons bypass ATP synthase—dissipates energy as heat rather than cellular currency, a hallmark of mitochondrial dysfunction observed in chronic fatigue and metabolic syndrome within the UK population.
Advanced INNERSTANDIN research highlights that efficiency is regulated by the mitochondrial dynamic cycle of fission and fusion. Mitophagy, the selective autophagic clearance of deleterious mitochondria, is essential for maintaining a high-functioning pool of organelles. When fission exceeds fusion—often due to chronic inflammatory signalling or systemic oxidative stress—the mitochondrial network fragments, leading to diminished bioenergetic output.
Furthermore, the role of NAD+ availability cannot be overstated. As a critical coenzyme for sirtuin-mediated mitochondrial biogenesis via PGC-1α activation, NAD+ levels directly correlate with the oxidative phosphorylation capacity. Our analysis suggests that metabolic recalibration, targeting the NAD+/NADH ratio, is the primary lever for enhancing mitochondrial coupling efficiency. By optimising the cristae morphology and maintaining membrane lipid homeostasis—specifically the saturation levels of cardiolipin—the cell minimises oxidative stress while maximising ATP throughput. Understanding these cellular mechanisms is paramount for INNERSTANDIN; it is not merely about energy production, but the orchestration of high-fidelity electron transport, ensuring that the human machine functions at the absolute threshold of its physiological potential, free from the entropic decay that characterises cellular senescence.
Environmental Threats and Biological Disruptors
The integrity of the mitochondrial reticulum is not an isolated affair; it is perpetually under siege by a suite of environmental stressors that actively undermine the stoichiometry of oxidative phosphorylation (OXPHOS). Within the context of INNERSTANDIN, we must recognise that mitochondria are the primary sensors of exogenous toxicity, and their subsequent dysfunction serves as the sentinel event for systemic metabolic pathology.
Primary among these threats are persistent organic pollutants (POPs) and endocrine-disrupting chemicals (EDCs), such as bisphenol A (BPA) and per- and polyfluoroalkyl substances (PFAS), which are ubiquitous in the UK water supply and food packaging. Research published in The Lancet Planetary Health underscores that these compounds act as uncouplers of the mitochondrial membrane potential. By intercalating within the inner mitochondrial membrane (IMM), these xenobiotics disrupt the proton gradient established by the electron transport chain (ETC). This dissipation of the electrochemical proton motive force compels the mitochondrion to increase oxygen consumption to compensate for the loss of ATP synthesis efficiency, inadvertently generating a surge of reactive oxygen species (ROS).
Furthermore, chronic exposure to fine particulate matter (PM2.5) represents a critical disruptor of mitophagic clearance. Recent toxicological data indicate that inhaled particulates translocate into the systemic circulation, where they trigger systemic inflammatory cascades. The ensuing oxidative stress leads to the peroxidation of cardiolipin—a unique phospholipid essential for the structural scaffolding of the ETC supercomplexes. When cardiolipin is oxidised, the cristae morphology destabilises, leading to the leakage of cytochrome c into the cytosol, a definitive precursor to programmed cell death.
The anthropogenic shift towards high-frequency electromagnetic field (EMF) exposure also warrants rigorous interrogation. Mechanistic studies archived in the National Library of Medicine suggest that non-ionising radiation may trigger voltage-gated calcium channels (VGCCs) located on the mitochondrial membrane. The subsequent cytosolic calcium overload induces mitochondrial permeability transition pore (mPTP) opening, which initiates a bioenergetic crisis. This is compounded by the synergy of ultramodern dietary glycotoxins—specifically advanced glycation end-products (AGEs)—which cross-link mitochondrial proteins, further impairing the enzymatic kinetics of the Krebs cycle.
For the INNERSTANDIN learner, it is imperative to grasp that these environmental stressors do not act in a vacuum. They establish a cumulative bio-burden that accelerates the age-related decline of mitochondrial biogenesis. As the PGC-1α master regulatory pathway becomes chronically downregulated by these stressors, the capacity for mitogenesis fails to keep pace with the rate of organelle degradation. Consequently, the human machine is forced into a state of chronic bioenergetic insufficiency, manifesting clinically as the metabolic syndrome epidemic currently overwhelming the NHS. Understanding these disruptions is the foundational step in reclaiming cellular sovereignty.
The Cascade: From Exposure to Disease
The transition from sub-optimal mitochondrial function to overt systemic pathology represents a complex bioenergetic collapse often overlooked in conventional clinical diagnostics. At INNERSTANDIN, we recognise that this decline is not an instantaneous event but a cascading failure of the electron transport chain (ETC) and its subsequent metabolic signalling. When the mitochondria—the primary engines of the human machine—suffer from diminished efficiency, the immediate consequence is an exponential increase in the leakage of reactive oxygen species (ROS) at Complexes I and III. Under physiological equilibrium, the mitochondrial membrane potential ($\Delta\psi_m$) maintains a precise gradient to drive ATP synthesis via oxidative phosphorylation (OXPHOS). However, exposure to chronic inflammatory triggers, environmental xenobiotics, or persistent metabolic stress induces mitochondrial uncoupling, effectively decoupling the oxidation of substrates from the phosphorylation of ADP.
This uncoupling is not merely a loss of energy; it initiates a destructive feedback loop. As ATP production falters, the resulting adenosine monophosphate (AMP) accumulation triggers the activation of AMP-activated protein kinase (AMPK), which, while initially compensatory, eventually contributes to metabolic inflexibility. Prolonged ROS efflux induces oxidative damage to mitochondrial DNA (mtDNA). Unlike nuclear DNA, mtDNA lacks the protective histone scaffolding and possesses a more limited repair capacity, rendering it highly susceptible to somatic mutations. As evidenced by research published in The Lancet, the accumulation of these mutations facilitates a decline in the structural integrity of the inner mitochondrial membrane, further exacerbating the leakage of cytochrome c into the cytosol.
This release of cytochrome c is the definitive trigger for the intrinsic pathway of apoptosis. When this process becomes dysregulated, it shifts from a programmed cell-clearance mechanism to a driver of chronic degenerative disease. In the context of the UK’s rising incidence of metabolic syndrome and neurodegenerative conditions, the failure to maintain mitochondrial homeostasis is central. The cascade flows from sub-cellular dysfunction to cellular senescence, where the accumulation of senescent cells—often termed "zombie cells"—secrete a pro-inflammatory secretome (SASP) that propagates mitochondrial damage to adjacent, previously healthy cells. This systemic propagation is the foundational mechanism behind the development of insulin resistance, mitochondrial myopathies, and the neuro-inflammation observed in Alzheimer’s pathology. INNERSTANDIN highlights this progression to emphasise that disease is not an external misfortune, but an end-point of an exhaustive internal bioenergetic decline. To intervene, one must look beyond symptoms and address the threshold where metabolic efficiency gives way to pathological entropy.
What the Mainstream Narrative Omits
The contemporary medical paradigm often reduces mitochondrial dysfunction to a terminal downstream symptom of genetic pathology or advanced neurodegeneration. However, the INNERSTANDIN perspective necessitates a shift in focus: we must recognise that mitochondrial efficiency—or the lack thereof—functions as the primary metabolic fulcrum upon which systemic homeostasis balances. Mainstream discourse frequently ignores the nuance of mitochondrial dynamics, specifically the interplay between fission, fusion, and selective autophagy (mitophagy), which govern the cellular energy currency.
The prevailing clinical narrative focuses disproportionately on ATP yield through oxidative phosphorylation (OXPHOS), essentially treating the mitochondrion as a static furnace. This reductionist approach neglects the reality of mitochondrial dynamics as a sophisticated signal-transduction network. Research published in The Lancet and various molecular biology compendia underscores that mitochondrial morphology is intrinsically linked to energy demand. Chronic metabolic inflexibility—the inability to shift efficiently between fatty acid oxidation and glucose utilisation—is not merely a lifestyle consequence; it is a profound failure of the mitochondrial reticulum to adapt its membrane potential ($\Delta\psi m$) in response to environmental stressors.
Furthermore, the mainstream narrative conspicuously omits the significance of the electron transport chain (ETC) leak, where electrons bypass the standard respiratory chain to form reactive oxygen species (ROS). While ROS are frequently demonised, biological research now confirms they are vital signalling molecules for mitohormesis—the process by which controlled mitochondrial stress induces long-term protective adaptations. By focusing purely on antioxidants as a palliative response to oxidative stress, mainstream medicine effectively blunts these crucial signalling pathways, preventing the cell from initiating necessary repair protocols.
At INNERSTANDIN, we argue that the critical oversight lies in the suppression of mitochondrial biogenesis via the PGC-1α pathway. When systemic inflammation persists, the cell downregulates the synthesis of new mitochondria, leading to an accumulation of damaged organelles that possess impaired mitophagy clearance mechanisms. This creates a feedback loop of metabolic inefficiency that precedes the clinical manifestation of metabolic syndrome. By failing to address the fundamental mechanics of mitochondrial quality control, modern physiological intervention remains tethered to symptom management rather than addressing the primary bioenergetic collapse that underpins modern chronic morbidity.
The UK Context
Within the contemporary British landscape, the precipitous decline in metabolic health is increasingly viewed through the lens of mitochondrial bioenergetics. Analysis of population-level data suggests that the prevalence of metabolic syndrome—a constellation of insulin resistance, visceral adiposity, and systemic inflammation—is fundamentally a pathology of impaired mitochondrial oxidative phosphorylation (OXPHOS). In the UK, where sedentary behaviour is coupled with an ultra-processed food environment, the resultant oxidative stress is forcing a re-evaluation of how we quantify cellular vitality. At INNERSTANDIN, we recognise that the mitochondria are not merely ‘powerhouses’; they are sophisticated signalling hubs that dictate cellular fate, apoptosis, and nuclear gene expression via retrograde signalling.
Clinical data published in The Lancet underscores the epidemiological reality that mitochondrial dysfunction is a primary driver in the accelerated ageing observed in deprived demographic cohorts across the UK. The mechanism is clear: chronic nutrient excess, specifically in the form of exogenous glucose and saturated fats, leads to an overload of the electron transport chain (ETC). This saturation causes an electron ‘leak’ at Complexes I and III, resulting in the excessive production of reactive oxygen species (ROS). These ROS induce mitochondrial DNA (mtDNA) mutations and compromise the structural integrity of the mitochondrial cristae, effectively decoupling respiration from ATP synthesis.
Research suggests that this bioenergetic failure is exacerbated by the depletion of specific micronutrient cofactors, particularly NAD+ and Coenzyme Q10, which are chronically low in the standard British diet. When the mitochondrial membrane potential ($\Delta\psi_m$) collapses, the cell shifts from efficient aerobic metabolism to less efficient anaerobic glycolysis—a state analogous to the Warburg effect. By integrating these physiological insights, INNERSTANDIN posits that the rectification of mitochondrial efficiency is the singular most potent intervention for reversing systemic decline. Bridging the gap between high-level biochemical research and clinical application is the only viable methodology to address the mounting crisis of chronic metabolic disease currently burdening our national health infrastructure.
Protective Measures and Recovery Protocols
The optimisation of mitochondrial bioenergetics necessitates a dual-pronged strategy: the mitigation of reactive oxygen species (ROS) mediated damage and the proactive stimulation of mitochondrial biogenesis. At the INNERSTANDIN research standard, we define efficiency not merely as ATP output, but as the maintenance of a robust mitochondrial membrane potential (ΔΨm) amidst systemic oxidative stress.
The primary mechanism for protecting the mitochondrial matrix is the endogenous upregulation of the Nrf2-ARE (Nuclear factor erythroid 2-related factor 2) pathway. Peer-reviewed data published in The Lancet and various molecular medicine journals confirm that chronic mitochondrial dysfunction—often stemming from sub-optimal electron transport chain (ETC) coupling—results in electron leakage at Complexes I and III. This leakage facilitates the formation of superoxide radicals. To counter this, one must prioritise the bioavailability of exogenous phytochemicals such as sulforaphane and resveratrol, which act as hormetic stressors, signalling the cell to ramp up mitochondrial superoxide dismutase (MnSOD) and glutathione peroxidase production. By modulating the Nrf2 pathway, we effectively neutralise oxidative insults before they trigger the opening of the mitochondrial permeability transition pore (mPTP), a catastrophic event that initiates cytochrome c release and subsequent apoptosis.
Regarding recovery protocols, the physiological demand for NAD+ precursors cannot be overstated. NAD+ serves as the essential substrate for sirtuin-mediated deacetylation of mitochondrial proteins, specifically PGC-1α (peroxisome proliferator-activated receptor-gamma coactivator 1-alpha). As the master regulator of mitochondrial biogenesis, PGC-1α orchestration is dependent upon the NAD+/NADH ratio. Current longitudinal studies suggest that supplementing with nicotinamide riboside or nicotinamide mononucleotide, combined with time-restricted feeding (TRF) protocols common in modern British nutritional research, significantly enhances mitophagy—the selective degradation of defective mitochondria. This "cellular housekeeping" is critical; failure to clear damaged mitochondria (mitophagy) leads to the accumulation of mutated mtDNA, which compromises the integrity of the respiratory chain and systemic metabolic throughput.
Furthermore, photobiomodulation (PBM) at the 660nm and 810nm spectra offers a non-invasive intervention for restoring cytochrome c oxidase activity. This enzyme, the final rate-limiting step of the ETC, exhibits a higher affinity for photons than for oxygen when inhibited by nitric oxide (NO) in high-stress states. By displacing NO, PBM effectively restores the proton gradient and enhances ATP production. Consequently, the INNERSTANDIN perspective maintains that mitochondrial efficiency is not a static biological parameter, but a dynamic, manageable metabolic state requiring precise pharmacological and environmental orchestration to preserve long-term cellular viability.
Summary: Key Takeaways
Mitochondrial efficiency represents the definitive nexus between metabolic homeostasis and the prevention of chronic degenerative pathologies. As underscored by data published in The Lancet, the efficacy of oxidative phosphorylation (OXPHOS) is intrinsically linked to the mitigation of mitochondrial reactive oxygen species (mROS) production, which serves as a primary driver of systemic cellular senescence. INNERSTANDIN maintains that optimising the electron transport chain—specifically the coupling efficiency of the inner mitochondrial membrane—is essential for sustained ATP production and the maintenance of membrane potential. Clinical evidence confirms that compromised mitochondrial biogenesis, often exacerbated by sedentary lifestyles and suboptimal nutritional substrates, precipitates metabolic flexibility deficits, insulin resistance, and neurodegeneration. By enhancing mitochondrial dynamics, including fission-fusion homeostasis and mitophagy, one effectively upgrades the bioenergetic architecture of the human organism. Ultimately, achieving peak mitochondrial function necessitates a rigorous, evidence-based approach to metabolic regulation, ensuring that every cell performs at its physiological zenith to withstand the oxidative stressors inherent to modern environmental exposures.
This article is provided for informational and educational purposes only. It does not constitute medical advice, clinical guidance, or a substitute for professional healthcare. Information reflects cited research at time of publication. Always consult a qualified healthcare professional before acting on any health information.
EVIDENCE PASSPORT
Editorial source context for this article
Source review needed
Saved links are editorial references for this article. They may support specific claims rather than every sentence. Open and assess each source in context. This passport does not independently verify them.
Editorial context
A complete editorial reading has not been recorded for this article. Source links remain available for you to open and assess directly.
Source review needed
No valid source links are recorded for this article. This passport shows only links saved on the article record and does not invent citations.
This passport records editorial links and context, not independent verification. Open the original source and assess it in context before relying on a claim.
Medical Disclaimer
The information in this article is for educational purposes only and does not constitute medical advice, diagnosis, or treatment. Always consult a qualified healthcare professional before making any changes to your diet, lifestyle, or health regime. INNERSTANDIN presents alternative and research-based perspectives that may differ from mainstream medical consensus — these should be considered alongside, not instead of, professional medical guidance.
Read Full DisclaimerContinue the thread
Keep this question moving.
Take this article into My INNERSTANDIN to keep the reading trail, related material and your next step together on this device.
Explore this in the Body Map
See where this hits your biology. Interactive anatomy, threats, and protective protocols.
Dig deeper in the Library
Free, longform PDF volumes that go beyond headlines into mechanisms and references.